In the context of climate changes, expected increases
in intensity, frequency, and unpredictability of waterlogging events
will aggravate wheat yield losses, currently estimated to range between
20-50%. Wheat production must fulfill ca. 20% of the population’s energy
and protein requirements. Evaluating germplasm with different
backgrounds may reveal variability for waterlogging tolerance, allowing a
better selection of genotypes with desirable traits for wheat breeding
programs. In this work, the effect of waterlogging on adventitious root
emission, tiller survival and yield was evaluated. Five studied
germplasm groups (Portuguese Landraces; Varieties with introduced
Italian germplasm; Post-Green Revolution varieties with introduced
CYMMIT germplasm; Advanced Lines from the Portuguese Cereal Breeding
Program; Australian varieties) were studied. Groups exhibited intra and
intervariability in all parameters in response to waterlogging imposed
in climatized growth chambers. After 14 days of waterlogging, the number
of adventitious roots ranged from 0 to 7.6 plant-1, with 4 Portuguese
Landraces depicting the highest number. The number of living tillers at
the end of the stress was highly variable, ranging from reductions of
100% to increases up to 35%. At harvest, the number of productive
tillers significantly differed among genotypes, with reductions reaching
100% in some cases and increases up to 138% in others. The existence of
variability and the identification of key traits underlying
waterlogging tolerance will contribute to develop more adapted wheat
plants and to improve wheat yield.
Keywords: Triticum aestivum L.; Portuguese Landraces; Australian varieties, CYMMIT germplasm; Advanced lines; Tillers; Excess water; Waterlogging
Abbreviations:
AdvL - Advanced Lines from the Portuguese Wheat Breeding Program; AR -
Adventitious roots; Austrl - Australian varieties; CP - Main culm; GR -
Post-Green Revolution varieties with the introduction of CYMMIT
germplasm; IT - Varieties with the introduction of Italian germplasm; K
nº - Kernel number; Pl - Plant; PL - Portuguese Landraces varieties;
Prod - Number of productive tillers at the end of the growth cycle;
Prod/Max - Ratio between Number of Productive tillers and Maximal number
of emitted tillers; SKW - Single kernel weight; T - Tillers; T0 -
beginning of waterlogging treatment; T2 - 2 days of waterlogging
treatment; T4 - 4 days of waterlogging treatment; T7 - 7 days of
waterlogging treatment; T7R - 7 days of recovery; T14 - 14 days of
waterlogging, end of waterlogging period; T14R - 14 days of recovery; WL
- plants subjected to 14 days of waterlogging; WW - control plants
As a result of climate change, the increased
instability of rainfall regimes raises the incidence of waterlogging
events [1-3]. Such stress currently affects 10 to 15 million hectares of
wheat-growing land, undermining food security as a result of
substantial yield losses (20 to 50%) [4]. This may compromise
approximately 20% of the world’s protein and energy needs, actually
ensured by wheat [5]. Waterlogged soil undergoes significant changes in
its chemical properties [6-8]. As the soil pores fill with water rather
than the gas phase, oxygen concentration is reduced which is exacerbated
by the drastic reduction of gas exchange between the soil and the
atmosphere [8,9]. The remaining oxygen trapped in the soil is rapidly
consumed by root respiration and by microbial activity in rhizosphere,
resulting in hypoxia or even environmental anoxia. Oxygen concentration
is inversely proportional to the Redox potential (Eh) value [10], and a
waterlogged soil typically displays a decrease in its Eh. According to
[11], a soil with an Eh
close to 0 mV will have an oxygen concentration of approximately
1%, leading plant roots to switch from aerobic to anaerobic
metabolism [8-11]. Thus, roots are the first plant organs to be
affected by hypoxia and anoxia due to waterlogging; resulting in
impaired root functioning and detrimental effects in shoots [12].
Waterlogging susceptible wheat genotypes frequently exhibit
severe metabolic constraints and growth arrest, enhanced leaf/
organ senescence, decreased accumulation and remobilization of
photoassimilates, and, reduced production [13-15]. The decrease
in yield is related with the number of kernels plant-1, spikes plant-1,
kernels spike-1, and the weight of a single kernel, which is reflected
in the thousand kernel weight.
Survival and development of tillers, as well as the ability
to produce new ones, are crucial traits in plants subjected to
waterlogging since they are directly proportional to the number
of spikes per area unit [16], with a direct effect on final yield [17].
Although a decrease in the number of emitted tillers occurs in
some varieties, this does not always reflect a decrease in fertile
ones, indicating some capacity to maintain production in an
energy deficit situation [17-19]. Nonetheless, the preservation of
the number of fertile tillers does not guarantee the maintenance of
yield, as their contribution to the final yield may be affected [16].
Several studies indicate that yield reduction due to waterlogging is
associated with low tillers survival [20-22] reduced fertile tillers,
and reduced kernel size [15,17]. The formation of adventitious
roots in response to waterlogging may be a strategy to reduce
oxygen deficiency, as these roots facilitate gas transport between
submerged tissues and the aerial portion of the plant. In addition,
these morphological adaptations play a decisive role in nutrient
and water uptake during waterlogging, significantly contributing
to survival [8,23] and to maintain productivity. The selection of
potential progenitors in breeding programs largely depends
on the evaluation and understanding of the existing genetic
variability [24,25]. Screening genotypes with distinct genetic
origins may provide the genetic diversity required for breeding
aiming to achieve crop yield stability and resilience in adverse
environments [26,27]. To understand the relationship between
the effects of a stress and its impacts on plant development,
studies conducted under controlled conditions provide the most
reliable and reproducible results [28].
The aim of this work was to evaluate, under controlled
conditions, the effect of 14 days of waterlogging on bread
wheat (Triticum aestivum L.) germplasm with distinct genetic
background. In each genotype, the effect of stress on adventitious
root formation, the number of surviving tillers during stress, after
recovery (7 and 14 days), and the fertile tillers obtained at the end
of the growth cycle, were evaluated. Final yield, kernel number,
and single kernel weight, were also evaluated per genotype,
as well as the contribution of the main culm and tillers in final
yield. Considering germplasm groups, the possible relationships
between the analyzed parameters were studied, along with the
interactions between the ability to emit adventitious roots and the
effects on the analyzed traits. The existence of variability and the
identification of key traits underlying tolerance to waterlogging
will contribute to develop more adapted wheat plants and to
improve wheat yield under a changing climate.
Wheat germplasm
The research focused on 23 wheat genotypes (Triticum
aestivum L.) from different origins and belonging to distinct
evolutive or breeding groups (Table 1): five Portuguese Landraces
(PL) from Vasconcellos ancient collection [29]; four varieties
released between 1950-1970 with introduced Italian germplasm
(IT) [30]; four Post Green Revolution varieties released between
1980-1989 with the introduced CIMMYT germplasm, according
to Almeida (2016) [30]; five Advanced lines from the Portuguese
Cereal Breeding Program (INIAV, I.P.) and five varieties from
Australian germplasm (Austrl). Certified seeds of each genotype
were provided by the Portuguese Cereal Breeding Program (INIAV,
Elvas, Portugal). Since limited amounts were available, seeds were
multiplied prior to the experiment, to ensure uniform germination
capacity (100%, results not shown) and adequate vigor of plant
material. This step was performed in growth chambers (Fitoclima
10000 EHHF, ARALAB, Portugal) under identical conditions of
temperature (22/15 oC, day/night), irradiance (ca. 800 μol m-2
s-1), relative humidity (70/75%, day/night), photoperiod (14 h),
and CO2 (400 μL L-1) in 5 L pots with field-collected loamy clay soil.
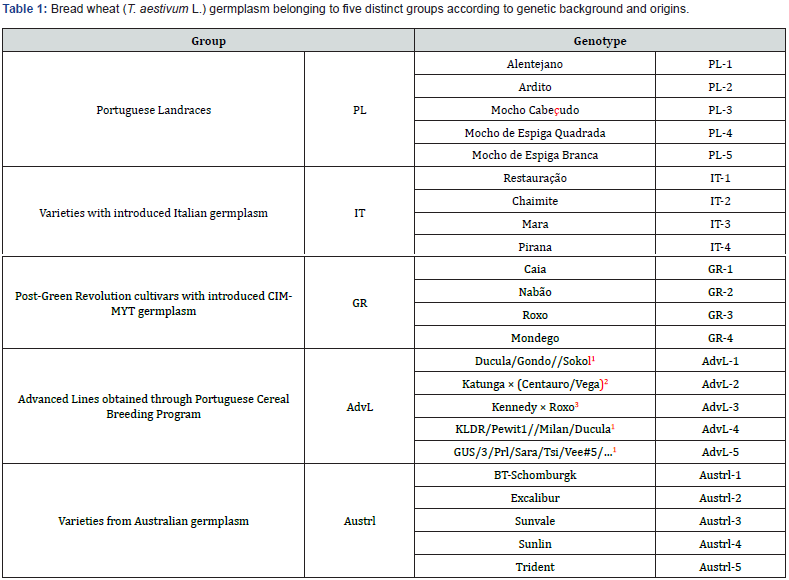
1CIMMYT material; 2Australian × Italian; 3Australian × Portuguese
Growth conditions
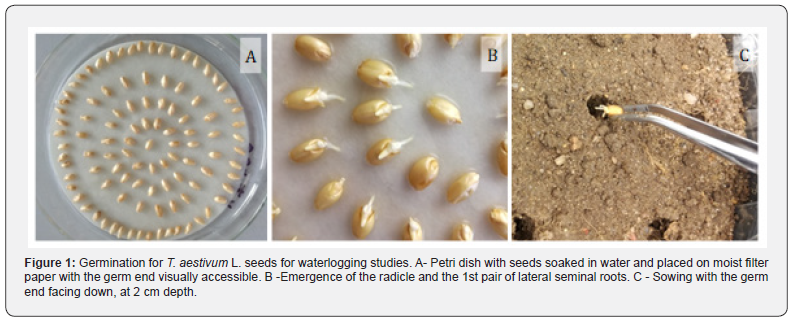
Approximately 120 seeds from each genotype were soaked
in water, placed on moist filter paper in Petri dishes (Figure 1A)
and kept at room temperature until the radicle and the first two
lateral seminal roots emerged (Zadoks scale 05 to 06, Z05 to Z06)
[31] (Figure 1B). The newly germinated seeds were then placed
at a depth of 2 cm (Figure 1C) with the germ end facing down, in
5L pots (7 seeds per pot) filled with sieved loamy clay soil. For
each genotype 12 pots (6 for control plants and 6 for waterlogged
plants) were prepared. Plants were grown in walk-in growth
chambers (EHHF 10000, ARALAB, Portugal), under controlled
temperature (22/15 °C, day/night), irradiance (ca. 500-600 μmol
m-2 s-1), relative humidity (75%), photoperiod (14 h) and CO2 (400
μL L-1) and maintained with a field capacity of ca. 85% except in
stressed plants during the waterlogging period. The plants were
fertilized weekly with 250 mL of a 12% N, 4% P, and 6% K solution
(Complesal, Bayer), except during waterlogging, the weeks
immediately preceding and following stress, and the final stages
of maturation.
Waterlogging imposition
When plants reached the tillering stage (Zadoks scale 22 to
25, Z22 to Z25) [31], half of the pots were kept at ca. 85% field
capacity (control plants, WW) and the other half were subjected to
waterlogging (waterlogged plants, WL). This was accomplished by
placing pots in plastic containers and flooding them until a water
layer of ca. 0.5 cm was formed above the soil surface. Daily, water
was added with care in order to maintain the water layer without
incorporating air. After 14 days, the water stress was suspended
by removing the pots from the boxes and maintained in the same
conditions as WW plants until harvest.
Soil Redox Potential (Eh)
Soil reduction-oxidation potential was measured in 1 pot of
each genotype in each treatment, at the beginning of waterlogging
(T0), after 24 h (T1), at 7 days of waterlogging (T7), at the end of
the stress period (T14) and after 7 and 14 days of recovery (T7R
and T14R, respectively). A portable Eh meter (XS-Instruments,
ORP-5, Italy) was used and measurements were performed at 6
cm deep and the value registered after its stabilization (ca. 15
minutes).
Adventitious roots
The number of adventitious roots was determined by
examining every plant in every pot at 2, 4, 7 and 14 days following
the onset of waterlogging (T2, T4, T7 and T14, respectively).
Number of tillers
The amount of living tillers was counted at T7, T14, T7R and
T14R in 18 plants per treatment. At the end of the growth cycle,
the number of productive tillers (Prod) was also obtained.
Yield
The impact of 14 days waterlogging in yield (g plant-1) was
evaluated in plants subjected to this stress as % of control plants at
the end of growth cycle. Plants were harvested and the productive
spikes counted and individually threshed.
Statistical Analysis
Data were analyzed using a two way ANOVA to evaluate the
differences between water treatments (WW or WL), between time
of treatments (T0, T2, T4, T7, T14, T7R, T14R and FC), and their
interaction, followed by a Tukey’s test for mean comparisons.
A 95% confidence level was adopted for all tests, which were
performed independently for each genotype using the software
PAST - Palaeontological Statistics software, version 3, University
of Oslo, Norway. For Pearson correlations, the same software was
used.
Soil redox potential
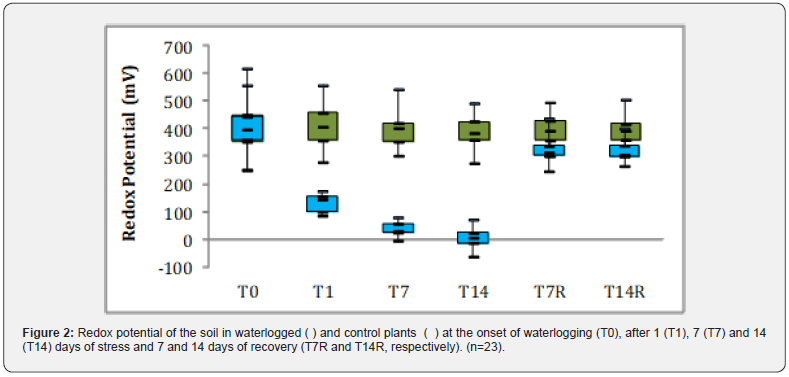
No differences in Eh values were observed between WW and
WL pots immediately prior to the imposition of waterlogging (T0).
In the pots that remained at ca. 85% field capacity, no changes
were observed between the observed periods (T0 to T14R) with
average values of ca. 400 mV, which is considered an ideal value
for plant development (Figure 2). In contrast, in the flooded
pots an abrupt decrease of Eh (due to the depletion of oxygen),
was observed earlier at T1, which was accentuated (although in
a softer way) in the following days, reaching minimum values
close to 0 mV (even negative in some pots). With waterlogging
suspension and the re-entrance of oxygen into the soil, Eh values
rose, approaching the values of WW pots after 7 days of recovery
(Figure 2).
Adventitious roots
Considering all genotypes, no adventitious roots (AR)
were
observed in plants grown under control conditions. However,
in plants subjected to waterlogging considerable heterogeneity
was detected within genotypes in each group, as well as between
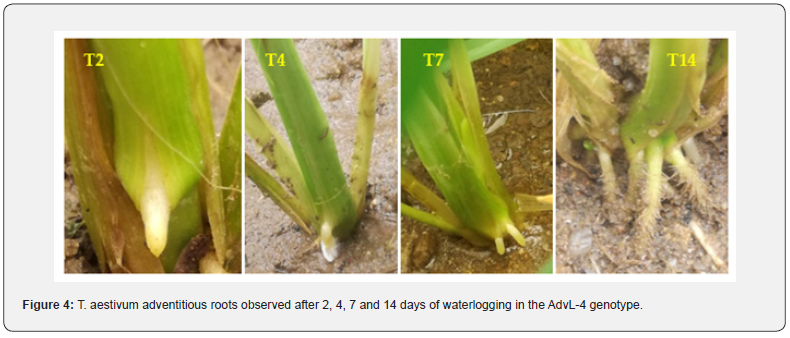
genotypes of the same group (Figure 3). With the exception of the
IT varieties, an early response (T2) in AR formation was observed
in some genotypes of the remaining groups (PL-1, PL-2, GR-2, Austrl-1,
Austrl-2, Austrl-3, AdvL-1, AdvL-4 and AdvL-5.) (Figures 3 & 4). In
contrast, AR were not formed in some genotypes (IT-3
and GR-4) or exhibited a very small number (IT-4, GR-1, GR-3 and
AdvL-3) at the end of the stress treatment (T14).
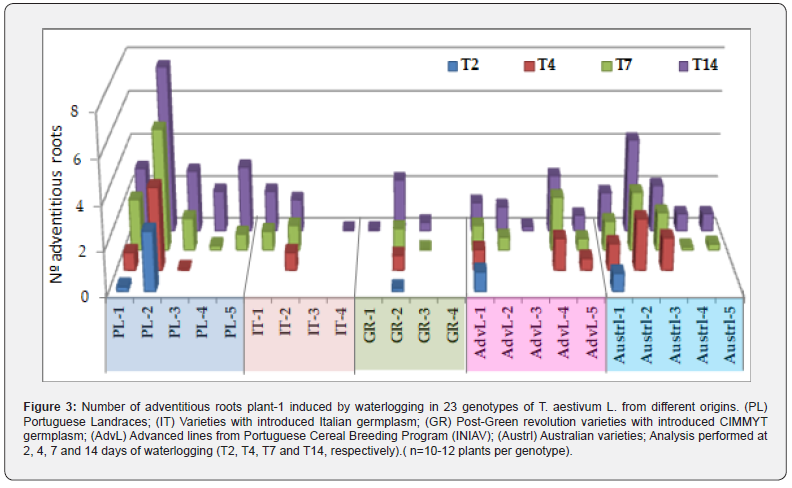
Across all analyzed WL periods, the PL-2 displayed the highest
number of AR per plant in comparison to the remaining genotypes.
At the end of the WL period (T14), this genotype presented a value
of 7.6 while a set of genotypes ranged from 4-2: Austrl-2 (4.3), PL-1
(3.6), PL-5 (3.3), PL-3 (2.9), AdvL-4 (2.6), GR-2 (2.4) and Austrl-3
(2.1). Another set showed values below 2 AR per plant (PL-4, IT-1,
Austrl-1, IT-2, AdvL-1 and AdvL-2) Nine genotypes exhibited less
than one AR per plant; Austrl-4, Austrl-5, AdvL-5, AdvL-3, GR-3. IT-
4, GR-1, IT-3 and GR-4, displayed values close to or equal to zero.
Tillers number and fertility
At the imposition of water treatment (T0), WW and WL plants
of all genotypes were in a similar phenological stage (Figure 5),
presenting 2-5 tillers (Z22-Z25) [31]. Regarding WW plants, a
great variability was observed in the average number of tillers
throughout the growth cycle (Figure 5). Although all plants of each
genotype had the same number of tillers at T0, there was some
variation in the tillers’ ability to survive, in plants capacity to emit
new tillers, as well as tillers fertility at harvest (Prod). At T7, the
number of living tillers ranged from 1.4 to 6.5, indicating either
the loss of some tillers (as in Austrl-4, AdvL-1 and AdvL-5) or, in
other cases, the progression of tillering (as in IT-3). This pattern
(reduction or increase in the number of tillers when compared
to T0) was observed in all germplasm groups throughout
observations conducted until the end of the growth cycle (T7, T14,
T7R, T14R, and Prod), with Prod corresponding to grain maturity
of productive tillers (Figure 5). Among germplasm groups, at T7,
the lowest value was found in Austrl while the highest in the IT
group. At T14 the number of tillers barely changed when compared
with T7. As the growing cycle progressed (T7R and T14R), both
the lowest values (1.3-1.7) and the highest values (7.4-7.7)
remained stable, with the first being found in the IT group and
the latter in the PL group. At harvest, there was variability in the
number of productive tillers between genotypes from distinct or
the same germplasm group. Prod values ranged from 0.5 to 1.9
for 12 genotypes and from 2.0 to 4.0 for 10 genotypes, from the 5
studied germplasm groups. Only AdvL-4 and Austrl-3 presented
more than 4 tillers (4.9 and 6.8, respectively). In contrast to
Austrl-3, which displayed the highest Prod value, AdvL-2 showed
the lowest value (0.5).
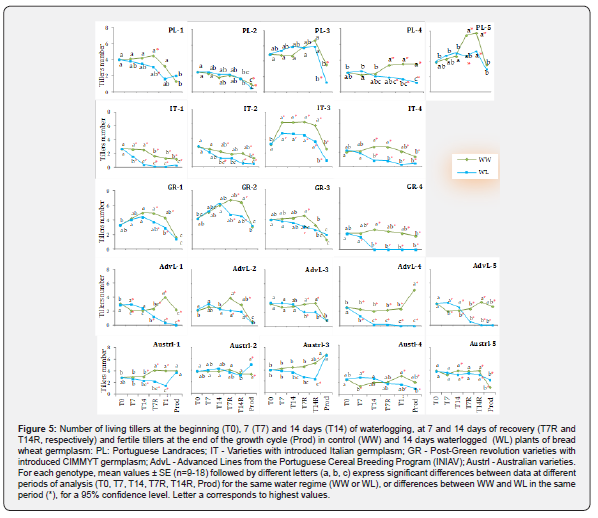
After 7 days of waterlogging (T7), the number of living tillers
in WL plants decreased in IT-1 (38%) and AdvL-4 (43%) (Figure
5), resulting in differences between WW and WL plants with
reductions in IT-1, IT-3, GR-4, AdvL-3 and AdvL-5, while Austrl-4,
AdvL-1 and AdvL-5 exhibited the opposite response with raises by
35, 43, and 61%, respectively. At the end of waterlogging (T14),
AdvL-5 was the only genotype presenting an increased number
of tillers (24%) in WL in relation to WW plants, in spite of 19%
(not statistically significant) decrease in WL plants between T7
and T14, denoting the death of tillers as waterlogging progress.
Despite some variations in the number of tillers, no waterlogginginduced
differences appeared in PL genotypes during this phase.
In contrast, the number of tillers decreased in all genotypes
of the IT group (27% to 84%) as well as in Austrl-1 (23%) and
Austrl-5 (18%). At T14, GR-4 presented no living tillers and AdvL-
4 presented a 90% reduction when compared with WW plants
(Figure 5).
The largest differences between WW and WL plants were
observed after 7 (T7R) and 14 (T14R) days of waterlogging
suspension. At T7R, 17 of the 23 genotypes significantly reduced
the number of tillers (24-100%) whereas at T14R, 18 genotypes
presented reductions between 18-100% (Figure 5). At T7R, WL
plants of the genotypes PL-2 and PL-3, IT-2, Austrl-2, Austrl-4 and
Austrl-5 had identical values to WW, while at T14R, there were
no differences between WW and WL in PL-1, PL-2, PL-3, in the
genotype GR-3, and in Austrl-2. At the end of the growth cycle,
some genotypes exhibited differences in the number of kernelproducing
tillers (Prod) (Figure 5). In the first group, PL-1, PL-2
and PL-5 were unaffected by waterlogging, whereas PL-3 and PL-4
showed 64 and 66% reductions, respectively. All of the genotypes
with Italian germplasm introduction were severely impacted by
water stress, with decreases of 68-88%. After recovery period,
GR-4 was the only genotype in its group to exhibit differences in
WL plants. All tillers died at T14 and it was unable to recover and
produce new tillers by the end of the cycle. Among the Australianorigin
germplasm, Austrl-1 and Austrl-3 were able to recover
from the damage suffered in T14 and during the recovery period,
displaying the same number of Prod tillers as plants not subjected
to waterlogging. The genotype Austrl-4 was negatively affected
with a 55% decrease in Prod tillers, while Austrl-5 and Austrl-2
showed an increase of 144% and 52%, respectively (Figure 5).
These two varieties were the only to exhibit this behavior among
the germplasm of the 5 groups under study. Similar to GR-4, the
AdvL-1, AdvL-4 and AdvL-5 did not recover and exhibited no Prod
tillers by the end of the growth cycle (Figure 5). The remaining
genotypes of this group did not differ in the number of Prod tillers
between WW and WL plants.
Considering that more tillers may result in more spikes at
harvest and that there were differences in tillering capacity among
the genotypes under study, we investigated whether waterlogging
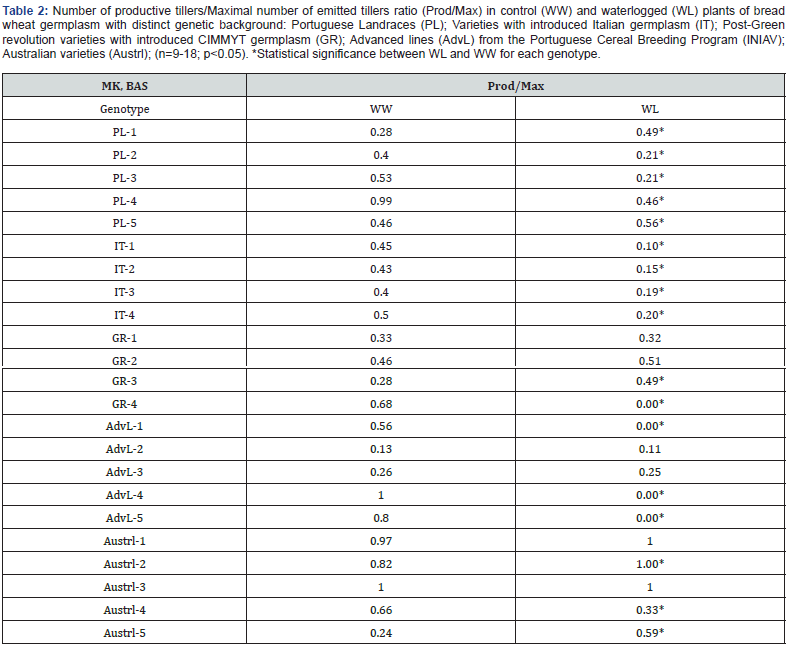
contributed to changes in the Number of productive tillers/
Maximal number of emitted tillers ratio (Prod/Max) (Table 2). In
addition to the observed variability in the number of tillers, the
Prod/Max ratio exhibited differences among genotypes and within
each germplasm group, for both WW and WL plants (Table 2). In
WW plants, PL-4, AdvL-4, Austl-1and Austrl-3 showed values of
1.0 or very close to it, while in 14 of the remaining genotypes, this
ratio was ≤0.5 (Table 2). As a result of waterlogging, Prod/Max
ratio decreased significantly in 12 genotypes, reaching 0 for GR-4,
AdvL-1, AdvL4 and AdvL-5. In contrast, this ratio increased in 5
genotypes (PL-1, PL-5, GR-3, Austrl-2 and Austrl-5), but was not
affected in seven genotypes, including the two Austrl (Austrl-1
and Austrl-3) with a ratio ca. 1.0 in WW plants.
Grain yield
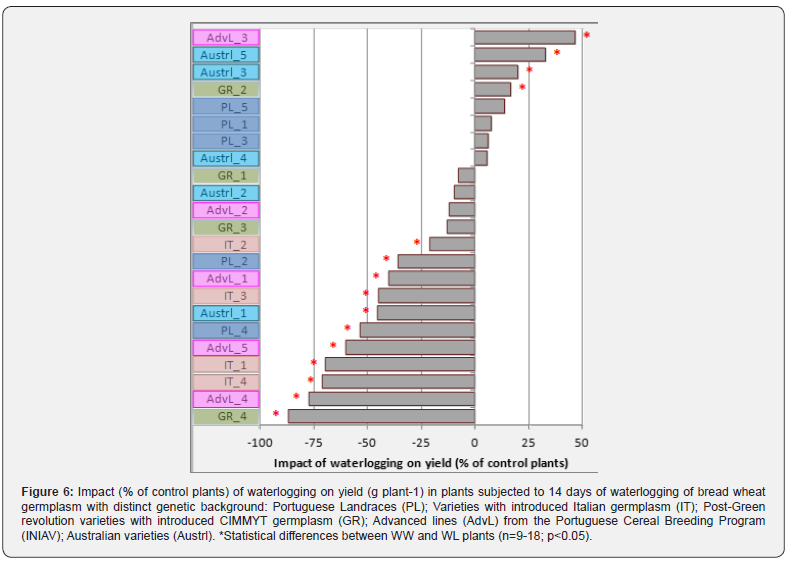
The majority of genotypes exhibited changes in yield due to
waterlogging (Figure 6). The genotype GR-4 was the most affected,
with an 87% reduction in yield, followed by AdvL-4 (77%). With
the opposite trend, AdvL-3 and Austrl-5 increased by 47 and 33%,
respectively, in response to waterlogging. Yield was negatively
affected by stress in the five groups (21 to 87% reductions
occurred in 11 genotypes), but the incidence was highest in the IT
group, where all genotypes showed yield decreases (21 to 71%).
Due to waterlogging, decreases, increases, and even no changes
were observed in the remaining groups (Figure 6). Yield decreases
appear to be related with the observed reduction in the number of
fertile tillers, but only in 8 of these genotypes. In the remaining 3,
decreased fertile tillers did not influence final harvest (Figure 6).
Grain yield
The majority of genotypes exhibited changes in yield due to
waterlogging (Figure 6). The genotype GR-4 was the most affected,
with an 87% reduction in yield, followed by AdvL-4 (77%). With
the opposite trend, AdvL-3 and Austrl-5 increased by 47 and 33%,
respectively, in response to waterlogging. Yield was negatively
affected by stress in the five groups (21 to 87% reductions
occurred in 11 genotypes), but the incidence was highest in the IT
group, where all genotypes showed yield decreases (21 to 71%).
Due to waterlogging, decreases, increases, and even no changes
were observed in the remaining groups (Figure 6). Yield decreases
appear to be related with the observed reduction in the number of
fertile tillers, but only in 8 of these genotypes. In the remaining 3,
decreased fertile tillers did not influence final harvest (Figure 6).
Genotypes that responded to stress with an augmented
number of fertile tillers showed a high yield, such as in Austrl-5
(47% yield increase), whereas the higher number of productive
spikes in IT-2 was accompanied by a 21% decrease in yield
(Figure 6). Among the three genotypes that recovered from severe
tillers mortality induced by waterlogging and in the 14 days that
followed, different yield results were observed. So, and despite
having the same number of fertile tillers as the WW plants, Austrl-
1’s yield was reduced by 45%. In contrast, GR-2 was able to achieve
a 17% increase (Figure 6). For genotypes that showed no change
in the number of living and fertile tillers, there was also important
variability in yield (Figure 6). In contrast to the increases observed
in AdvL-3 (47%) and Austrl-3 (33%), PL-2 experienced a 36%
decrease in yield despite a stable number of tillers. For PL-1, PL-5,
GR-1, and AdvL-2, maintaining the number of tillers also resulted
in an unchanged yield (Figure 6).
Root features determine plants ability to absorb water and
nutrients for their growth, development and grain production
[8,32,33,34]. Adventitious roots play a crucial role to overcome
nutrient deficiency, providing an increased capacity to adapt
to different environments [35,36]. Given that a greater number
of adventitious roots may help the plant above-ground portion
to better cope with the negative effects of waterlogging [37],
tolerance seems to be closely linked to the ability to generate these
roots [38]. In response to waterlogging, PL and Austrl varieties,
considered the most tolerant among the tested germplasm,
exhibited the largest number of adventitious roots (AR). The PLs
exhibit the genetic heterogeneity of regional varieties [30] and are
part of a wheat germplasm collection [29] that had been grown
for generations in Portugal. These locally adapted cultivars are
considered a valuable source of variability for breeding programs
[27]. As the root system plays a major role in waterlogging
conditions, landraces appear to be a solid option for selecting and
crossing parental genotypes depicting beneficial root features,
aiming the obtention of more adapted ideotypes [27]. In PLs,
the ability to emit AR was accompanied by heterogeneity among
varieties, both in the number of AR and in emission precocity. This
heterogeneity is expected in landraces [27] and constitutes an
asset for breeding programs. In Portugal, wheat breeding program
has gone through several phases. Between 1950 and 1968, the
introduction of Italian germplasm (IT Group) led to the release
of the 1st Portuguese variety (Pirana, IT-4). Since the early 60’s
a strong cooperation with CYMMIT led to the introduction of
germplasm with dwarfism (Rht) genes. Observing also the current
advanced lines from the Portuguese Cereal Breeding Program,
apparently wheat genetic improvement has not led to a loss of
variability in plant root characteristics, namely in root growth
angle [33] or the ability to emit adventitious roots in response
to waterlogging, as suggested by the results of this study. The
observed genotypic variability in AR emission is in agreement with
reported results, where wheat sensitive varieties to waterlogging
had fewer AR than those tolerant to this stress [32,39].
Regarding tiller number, waterlogging generated decreases
(although at different times) in all genotypes, except for PL-1
and Austrl-2, which remained stable. This reduction is consistent
with results reported by several authors [17,19,32,40,41,42,43].
However, variability in response to waterlogging was observed.
Some genotypes showed an early and strong tiller growth arrest at
T7, extended until harvest (IT-1, IT-3, GR-4, AdvL-4), causing severe
yield decreases and denoting no tolerance to waterlogging. Other
genotypes showed a similar pattern but only from T14 onwards,
namely IT-2 and IT-4. Results indicated that all genotypes of IT
group were affected with significant reductions in yield (21-71%).
With the end of waterlogging, 20 genotypes displayed decreased
tillers number at recovery (T7R and/or T14R), suggesting a
deleterious effect when oxygen availability is reestablished. This
might cause the formation of reactive oxygen species (ROS) due
to O2 re-entry in plant tissues, leading to cell membrane damages
[40].
In wheat, tillering can occur during the entire
growth cycle
[44]. In this study, 6 genotypes (PL-1, PL-2, Austrl-1, Ausrl-2,
Austrl-3 and Austrl-5) were either unaffected or were able to
generate new tillers, achieving values comparable to those of
the control plants, or even higher, at the end of growth cycle.
According to Xie (2016) [45], tillering ceases just prior to
elongation and the remaining axillary buds become dormant. This
dormancy, however, can be reversed in response to damage to the
main shoot or lodging [46], which is consistent with the observed
results and point to some genotypic variability regarding recovery
ability following waterlogging Decreased tillers viability may also
result from nutrient resources remobilization from late tillers to
primary tillers [47]. Additionally, tillers can serve as reservoirs
of assimilates for the main culm during growth cycle [48]. This
might explain the low tillers value observed in some genotypes
(e.g. AdvL-2), reflecting the death of the majority of tillers even
under controlled conditions and an emphasis on the main culm’s
major contribution to the final yield. Thus, the number of tillers
is not necessarily an indicator of fertile spikes being produced.
Regarding the Number of productive tillers/Maximal number of
emitted tillers ratio (Prod/Max) found for control plants, values
are consistent with reports from several authors, who described
average mortality rates of 10-80% of all initiated tillers [45,49,50].
Waterlogging strongly influenced the Prod/Max in some genotype,
which reached zero in 4 genotypes, reflecting the mortality of all
emitted tillers, or values ≤0.5 indicated that half or less of the
produced tillers reached maturity, with drastic repercussions on
yield. Many studies reported reductions of up to 66% of tillers
at maturity when waterlogging was imposed at tillering stage
[18]. Among germplasm considered in the present work, several genotypes
displayed an increased or unchanged Prod/Max ratio, denoting a good
capacity to invest in fertile tillers, even under
adverse conditions. Robertson (2009) [19] reported that under
waterlogging imposed at tillering, some genotypes reduced the
number of initiated tillers, although at maturity presented similar
values to WW plants. On the other end, some genotypes started
emitting new tillers when waterlogging ended [32].
Yield losses in waterlogged plants ranged from 21% to 87%,
which is consistent with values from other studies (ca. 30% to
90% decreases), namely on wheat [18,40,44,51,52,53,54]. Such
reductions were observed in 11 genotypes and appear to be
closely linked to all tillers death (GR-4, AdvL-1, AdvL-4 and AdvL-
5) or decreased tillers survival. Several authors observed yield
reductions under waterlogging as a result of low tiller survival
[15,17]. In addition, fewer kernels per spike [19,41,43,55,56] and
smaller tillers and kernels [20,21,22], can also negatively affect
final yield [16] and must be addressed in future work. The present
results highlight 4 genotypes with yield increases in waterlogged
plants and 8 that were unaffected by stress. Tian (2021) [57]
reviewed the overall change in crop yield induced by waterlogging
in 115 studies and found that this stress can increase, decrease or
maintain crop yield. They also suggested that this could be due
to differences in crop varieties tolerance or sensitivity to shorter/
prolonged waterlogging periods.
This study in bread wheat revealed significant variability in the
number and precocity of adventitious roots formed in response
to waterlogging, as well as in tillering survival and emission
capacity. Such variability was reflected in the observed different
yield changes due to 14 days of stress imposed at tillering stage.
Differences between germplasm groups from different origins,
and within groups, may be a source of genetic material to develop
new varieties with distinct root system morphologies, to address
climate change-related issues.
Wheat tolerance to abiotic factors is a very important
breeding objective under changing climate. This study highlighted
variability in adventitious roots (AR), number of tillers and
yield in response to waterlogging at tillering stage, in 23 bread
wheat genotypes with different genetic backgrounds. Variability
occurred between and within the germplasm groups. AR were
formed only in plants subjected to stress and differences were
found in their number, with a few genotypes showing also earlier
AR emission. With waterlogging, some genotypes tillers were
affected with effects in final yield. The recovery period seems to
be the most critical, with 20 of the 23 genotypes being negatively
affected in living tillers number, probably due to oxidative stress
onset during aerobic conditions reestablishment. Overall, the
PL and Austrl genotypes performed better under waterlogging
conditions, while IT genotypes showed an opposite behavior. The
large variability found under the studied waterlogging conditions
suggests that the selection of tolerant genotypes should focus not
only the group they belong to, but also the germplasm as a whole.
To Know more about Agricultural Research & Technology: Open Access Journal
Click here: https://juniperpublishers.com/artoaj/index.php
To Know more about our Juniper Publishers
Click here: https://juniperpublishers.com/index.php